Nutrition
The Strongman Metabolism: Episode 5 - Mitochondria and Energy Production
September 7, 2026
The Strongman Metabolism: Episode 5 - Mitochondria and Energy Production
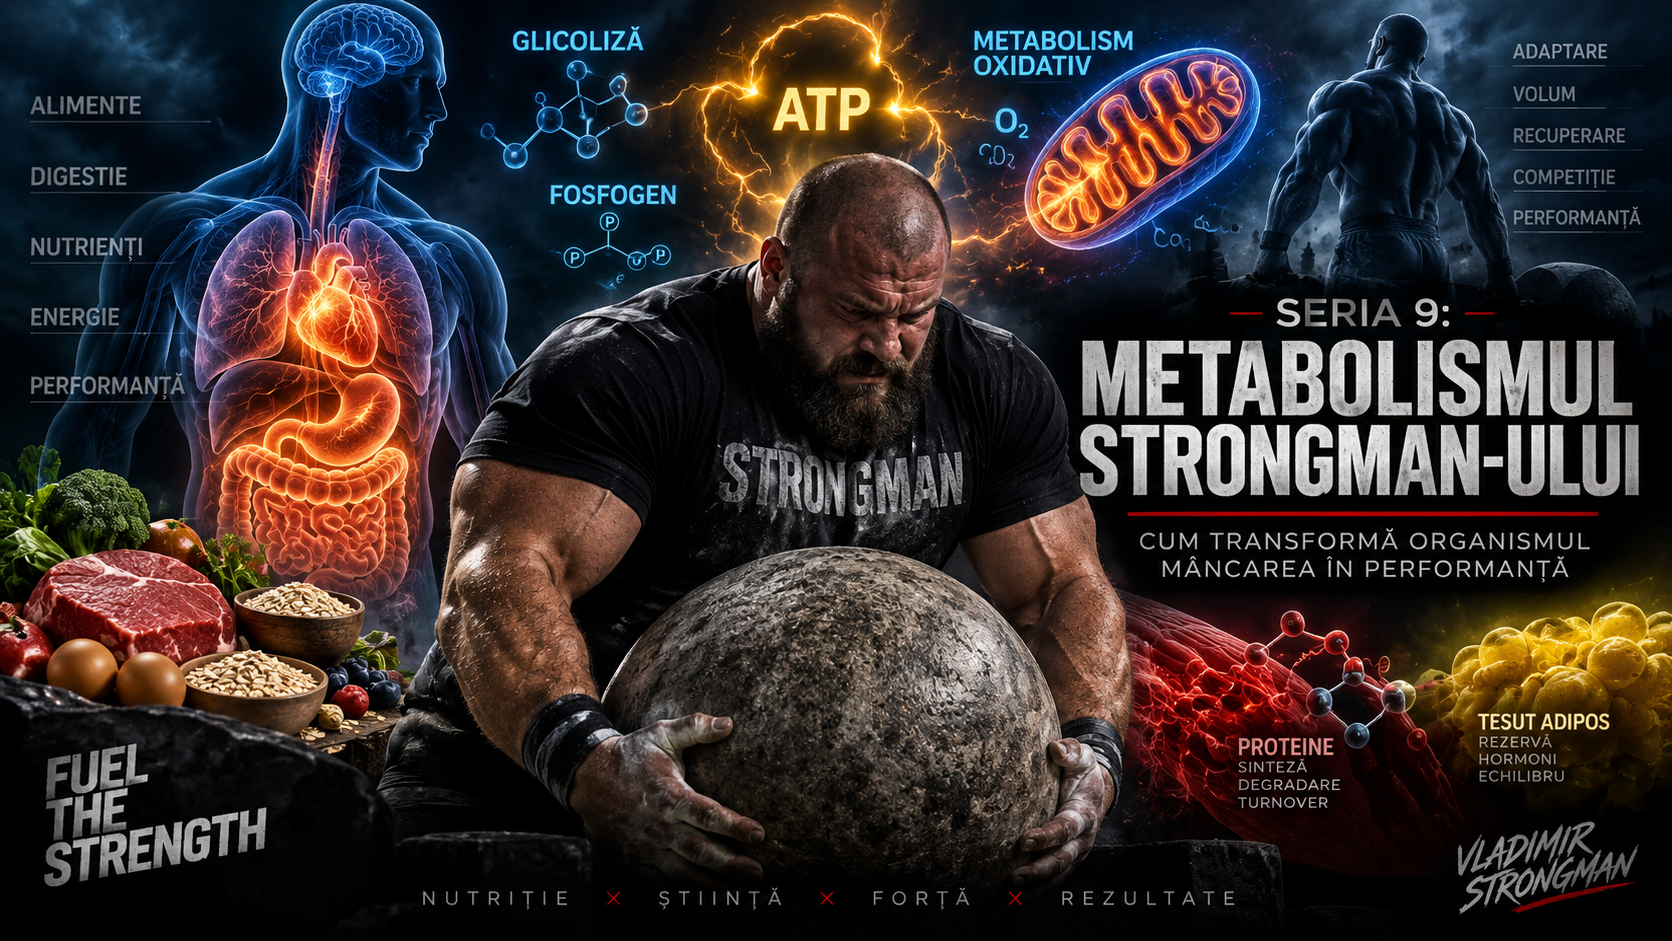
In the first four episodes of this series, we followed ATP, the phosphagen system, glycolysis and oxidative metabolism. Now we go one level deeper, into the cell, where chemical energy from food is converted into a usable flow of ATP. For a strongman, the mitochondrion is not a biology footnote. It is part of the machinery that determines how much work can be sustained and how quickly the body can recover after an event that has emptied its immediate energy reserves.
When you watch an athlete load an atlas stone, accelerate with farmer implements or repeat heavy loading reps, the eye sees mechanics. Inside the muscle fiber, an entire energy economy is running. ATP is consumed, ADP rises, phosphocreatine is used and then restored, carbohydrate enters glycolytic pathways, fat is broken down, and electrons reach the mitochondria. There, the respiratory chain creates the conditions required for continuous ATP resynthesis.
Why go all the way down to the mitochondrion?
It is tempting to summarize everything with the phrase “the mitochondria produce energy.” That is broadly correct, but it misses the architecture of the process. Mitochondria are metabolic hubs. They receive products from several pathways, extract electrons, create a proton gradient, synthesize ATP and participate in substrate oxidation, cellular signaling and adaptation to exercise.
This matters in strongman because event duration and the spacing between events change the problem. In one maximal rep, the rate of ATP delivery is the priority. In a long set, a medley or a competition day with several events, the ability to keep producing ATP and to restore what was spent becomes increasingly important.
ATP: currency, not a huge reservoir
In the earlier episodes, ATP was described as the energy currency. Take that idea one step further. The muscle contains only a relatively small immediate pool of ATP that must be recycled continuously. The body does not store a massive tank of ATP that it opens at the start of competition and drains to empty. ATP molecules are constantly broken down and rebuilt.
When myosin uses ATP during contraction, ADP and inorganic phosphate are produced. For the fiber to continue producing force, ADP must again become ATP. The phosphagen system can do this extremely quickly using phosphocreatine. Glycolysis can supply ATP rapidly. Mitochondria can sustain a lower but longer-lasting rate of oxidative ATP production.
How food energy reaches the mitochondria
Carbohydrates, fats and proteins do not enter mitochondria in the same form in which we eat them. They are processed through a sequence of reactions into intermediates that can feed oxidative pathways. Carbohydrates can be converted into pyruvate and then acetyl-CoA. Fatty acids enter beta-oxidation, generating acetyl-CoA, NADH and FADH2. These molecules are, in a useful sense, the deliveries arriving at the mitochondrial factory.
This helps explain metabolic flexibility. The body does not have one fuel. It has several sources and several entry points. What changes is how quickly each source can meet energy demand and what metabolic cost is involved.
Pyruvate: the intersection between glycolysis and mitochondria
Glycolysis converts glucose to pyruvate. Depending on cellular conditions and energy demand, pyruvate can be converted to lactate or can enter the mitochondria and be converted to acetyl-CoA by the pyruvate dehydrogenase complex. This step directly links glycolysis to the Krebs cycle and then to the respiratory chain.
For strongman, the link is essential. Glycolysis is not an isolated pathway that simply ends when lactate appears. Glycolytic products can continue into oxidative metabolism. During intense effort, these processes operate together, and their relative contribution changes constantly.
The Krebs cycle: the station that prepares the electrons
Acetyl-CoA enters the citric acid cycle, also called the Krebs cycle. A sequence of reactions processes carbon and generates reduced molecules, especially NADH and FADH2. These molecules are critical because they carry high-energy electrons toward the respiratory chain.
The Krebs cycle is not just a one-way conveyor belt. It is connected to carbohydrate, fat and amino-acid metabolism. Its intermediates can be withdrawn for other cellular functions and replenished by anaplerotic reactions. For an athlete, this means energy metabolism is linked with tissue maintenance, repair and synthesis, not only ATP production.
NADH and FADH2: the electron carriers
NADH and FADH2 act as carriers delivering electrons to the respiratory chain. The electrons enter at different points, and their energy is used to pump protons across the inner mitochondrial membrane.
That separation of charge creates an electrochemical difference. The mitochondrion uses the proton gradient to drive ATP synthase. In practical terms, the respiratory chain converts the energy of nutrient-derived electrons into a form that can be used to make ATP.
The respiratory chain: four major complexes and one simple idea
The mitochondrial respiratory chain contains protein complexes and mobile carriers. Complexes I, III and IV contribute to proton pumping, while complex II transfers electrons into the chain without pumping protons in the same way. Oxygen serves as the final electron acceptor at complex IV.
For the athlete, the core message matters more than memorizing the numbers: electrons from nutrients move through an energy-transfer system, and the resulting energy creates the gradient that powers ATP synthesis.
Oxygen: not the fuel, but the final acceptor
Gym language sometimes says that oxygen “burns” fuel. As a metaphor it is useful, but biochemically oxygen is the final electron acceptor in the respiratory chain. At the end of the process, electrons and protons contribute to the formation of water.
Without this final step, normal electron flow through the respiratory chain cannot continue. This is one reason oxygen transport and oxygen use matter so much in prolonged effort. The cardiovascular system delivers oxygen to tissue, and the mitochondria use it at the final stage of oxidative energy production.
The proton gradient: the mitochondria’s electrochemical battery
Pumping protons across the inner mitochondrial membrane creates a difference in concentration and electrical charge. This is the proton-motive force. ATP synthase allows protons to flow back across the membrane, coupling that energy to ATP synthesis.
This is the beauty of the mechanism: the cell does not turn a piece of glucose directly into ATP in one step. Energy is transferred in stages, and the mitochondrion manages an electrochemical system. For the athlete, the final product is ATP available for muscle contraction.
How much ATP does oxidative metabolism produce?
In broad terms, complete oxidation of glucose yields far more ATP than glycolysis alone. Exact values vary with electron-shuttle pathways and cellular conditions, which is why modern sources use approximate values. The main idea is that oxidative metabolism extracts a large amount of usable energy from substrate and can sustain production for long periods.
For a strongman, an isolated number is not the key point. What matters is that the mitochondria can keep recycling ATP long after the immediate phosphocreatine contribution used during the opening explosion has begun to fall.
Fat: slower entry, large energy yield
Fatty acids are an important oxidative energy source. They must be mobilized, transported and processed through beta-oxidation before their products enter the Krebs cycle and then the respiratory chain.
This route has a large energy capacity, but it cannot meet an extreme energy demand as quickly as phosphocreatine and carbohydrate-based pathways. As intensity rises, the relative contribution of carbohydrate therefore tends to become more important.
Carbohydrate: the fuel for intensity and continuity
Carbohydrate has a special role in intense effort because it can feed glycolysis quickly and supply pyruvate for oxidation. Muscle glycogen is directly accessible to the working fiber, making it highly relevant during training and competition where energy demand is high.
It is a mistake to oppose oxidative metabolism and carbohydrate. Carbohydrate oxidation occurs in the mitochondria. An athlete can use carbohydrate and produce ATP oxidatively at the same time. The real question is which substrate predominates and how quickly energy can be supplied.
What happens when ATP demand exceeds oxidative capacity?
During an explosive effort, ATP demand can rise faster than oxidative phosphorylation can respond. The high-rate systems, especially phosphagen and glycolysis, therefore contribute strongly. This does not mean the mitochondria switch off. They continue working, but their relative contribution is smaller compared with total instantaneous demand.
That distinction is central in strongman. An athlete can have good oxidative capacity and still need the phosphagen system for an explosive start. Another athlete can have excellent maximal strength but fade during a long set because the rate of energy restoration cannot keep up with demand.
Mitochondria and phosphocreatine recovery
After intense contraction, phosphocreatine has to be restored. That restoration requires ATP, and a large share of the ATP needed during recovery is supplied through oxidative metabolism. This creates a direct link between aerobic conditioning and repeated explosive performance.
If the gap between efforts is long enough, phosphocreatine can recover substantially. If the break is short, the next effort begins while some of the reserve is still depleted. Good oxidative capacity can accelerate energetic recovery, even though it does not make recovery instantaneous or complete.
The mitochondria and the strongman medley
In a medley, the athlete changes mechanics and dominant muscles, but the organism does not reset. The heart keeps pumping, ventilation remains elevated, phosphocreatine is partially restored and mitochondria keep producing ATP.
An athlete moving from sled to farmer carry and then to a loading implement has to meet several demands without full recovery between them. Oxidative capacity is one component that allows continued ATP production and faster recovery between bursts.
Mitochondria and repeated heavy loading
Imagine a loading set in which every repetition demands a powerful contraction but only a few seconds separate reps. The first repetitions may look almost identical. Then the pace slows. Grip changes. Breathing becomes harder. The athlete spends more time between reps.
The mitochondria do not rescue the set by themselves. They are part of the system that produces ATP between bursts and restores energetic capacity. The better prepared the oxidative machinery, the larger the margin for repeating high-intensity actions.
Mitochondria adapt to training
Mitochondria are not fixed structures. Training can alter mitochondrial density, oxidative enzymes, network organization and the muscle’s ability to use oxygen and substrates. In simple terms, a trained muscle can become better equipped to produce ATP oxidatively.
Adaptation is not instant. It emerges from repeated stimulus and adequate recovery. That is why conditioning should be evaluated over weeks and months, not by how destroyed one session makes you feel.
Mitochondrial biogenesis: building the infrastructure
A central concept in exercise physiology is mitochondrial biogenesis, the process through which cells expand and remodel their mitochondrial population. Training activates signaling pathways that alter the expression of genes involved in oxidative metabolism.
For strongman, the goal is not “more mitochondria at any cost.” The goal is enough oxidative adaptation for the demands of the sport while preserving recovery resources for strength, hypertrophy, technique and event training.
PGC-1α and the adaptation signal
PGC-1α is a well-known regulator of oxidative adaptation. Endurance training and other forms of metabolic stress can increase activity in this pathway, which influences expression of genes involved in mitochondrial biogenesis and oxidative metabolism.
For the athlete, this shows that training sends a message to the cell. Exercise is not merely calorie expenditure. It is biological information telling the body what kind of machinery it needs to build.
Mitochondria differ between muscle fibers
Muscle fibers differ in contractile and metabolic properties. More oxidative fibers tend to have higher mitochondrial density and capillarization and are well suited to aerobic energy production. Fast fibers specialize in force and power, but they also possess oxidative capacity.
A strongman needs a combination. The goal is not to make every fiber resemble that of an endurance athlete. The athlete needs access to strong, fast contractions while maintaining enough oxidative infrastructure to repeat the work.
The mitochondrial network: not just the number of mitochondria
Mitochondria form a dynamic network inside cells. Fusion and fission help maintain and remodel that network. Functional quality can therefore matter as much as quantity.
In a trained muscle, the exchange of substrates and energetic products is supported by a more capable metabolic infrastructure. That means we should not ask only how many mitochondria a muscle contains. We should also ask how well the network can produce and regulate energy.
Capillarization and mitochondria: one integrated system
Mitochondria need oxygen and substrates. Capillaries bring blood close to the muscle fiber, and diffusion allows gas and metabolite exchange. Oxidative adaptation therefore cannot be reduced to the organelle itself. Delivery to the fiber and use inside the cell are parts of the same system.
For strongman, these adaptations can become relevant in carries and sessions where work duration increases. A muscle that receives and uses oxygen effectively can maintain oxidative ATP production and manage repeated effort more effectively.
Mitochondria and lactate
Lactate is not simply waste that the body must throw away. It can move between tissues and be used as an oxidative substrate. Muscle fibers with high oxidative capacity can use lactate as fuel.
This changes how we interpret the so-called “lactic acid” story. Muscle burn does not mean lactic acid has filled a reservoir and switched the mitochondria off. During exercise, lactate production, transport and oxidation can occur at the same time.
Reactive oxygen species: the difficult side of oxygen
Oxidative metabolism also produces reactive oxygen species. They are not automatically harmful. They can act as signals involved in training adaptation. The problem arises when oxidative stress exceeds the capacity of antioxidant and repair systems.
The body has its own antioxidant systems, including enzymes such as superoxide dismutase, catalase and glutathione peroxidase. The aim is not to eliminate reactive species completely, but to maintain a balance that allows useful signaling without excessive damage.
Why we should not eliminate every form of stress
It is easy to treat every free radical as an enemy and every high-dose antioxidant strategy as a solution. Exercise physiology is more nuanced. Some of the stress generated by training is the signal that tells the body to adapt.
This is part of the idea of hormesis. A stimulus can be large enough to provoke adaptation while remaining controlled enough to allow recovery. In strongman, the principle applies to the whole program: stress, recovery and adaptation.
Mitochondria and heat
Not all chemical energy from nutrients becomes ATP. Some is released as heat. During exercise, this contributes to rising body temperature and the need for thermoregulation.
For a strongman, especially an athlete with high body mass competing in hot conditions, thermoregulation matters. Efficient mitochondria support energy production, but the body must also manage the heat generated by metabolism.
A long event starts with ATP and ends with ATP recovery
In a prolonged event, ATP is consumed from the first second. Phosphocreatine contributes immediately, glycolysis rises, oxidative metabolism contributes more as time passes, and after the event the body continues using ATP to restore internal order.
That continuity matters. Metabolism does not stop when the clock stops. Much of the invisible work that makes the next performance possible begins precisely then.
Between events: the mitochondria work backstage
Imagine a competition with a dynamic deadlift, then farmer carry, then a loading medley. Each event leaves a cost behind. Between them, the body has to restore phosphocreatine, process metabolites, normalize ventilation and circulation, replenish substrates and manage temperature.
Mitochondria are part of the machinery supporting that recovery. They do not determine recovery alone. Sleep, nutrition, hydration, the nervous system and tissue damage also matter. But oxidative ATP production is a major source of the energy required for many recovery processes.
VO2max versus mitochondrial capacity
VO2max reflects maximal oxygen consumption across the whole system. It is not synonymous with mitochondrial function. An athlete can have excellent central cardiovascular adaptations and still have peripheral limitations at muscle level. Conversely, muscular adaptations can improve oxygen use without every part of the system changing to the same degree.
For strongman, VO2max does not need to become an absolute target. What matters is building enough capacity to sustain the workload and recover according to real competition demands.
How to train mitochondria without sacrificing strength
The first principle is dosage. Low- or moderate-intensity sessions can provide an oxidative stimulus with manageable mechanical cost. Cycling, ergometers, incline walking and sled dragging can be useful for large athletes because they allow conditioning volume without the same joint loading as a heavy event circuit.
The second principle is specificity. As competition approaches, intervals and events can reproduce relevant work-to-recovery combinations. But specificity does not mean every session must be an exact competition simulation. Sometimes the best choice is a tool that develops the system at a lower cost.
Intervals and oxidative stress
Intervals create a work pattern in which intense effort is followed by incomplete recovery. Heart rate and ventilation remain elevated, and metabolism has to restore ATP in a context where demand returns before full recovery.
This can be a useful stimulus for strongman because many events resemble a sequence of bursts rather than one continuous linear effort. However, intervals must be dosed so they do not destroy the main strength days.
What is a “good” mitochondrion for a strongman?
It does not automatically mean the greatest possible mitochondrial density. It means enough oxidative capacity to produce ATP, use substrates, support repeated work and contribute to recovery without consuming excessive recovery resources.
A good strongman does not need to become a marathon runner. He needs enough conditioning that strength and body mass remain usable across a long competition day.
Nutrition and the mitochondria
Mitochondria require substrates and cofactors. Adequate energy intake, carbohydrates, fats, protein, vitamins and minerals support metabolic processes. Severe restriction and chronically low energy availability can reduce training and recovery capacity.
For a strongman, the message is simple: you cannot demand high output from a metabolic engine while continually starving its fuel supply. Nutrition does not magically switch mitochondria on, but it provides the materials and physiological context needed for function and adaptation.
Creatine and mitochondria: complementary systems
Creatine and phosphocreatine belong to the fast-energy story developed in the first episodes. Mitochondria operate on a different time scale. One system supplies the immediate explosion, while the other supports longer-term energy production and recovery infrastructure.
That complementarity is exactly what strongman demands. You need to produce force now and produce it again seconds later, minutes later or in the next event. The energy systems are not rivals. They are components of the same circuit.
Mitochondria and muscular efficiency
A muscle with strong oxidative adaptation can use oxygen and substrates efficiently and maintain a more stable energy flow during submaximal and repeated work. This does not automatically make the athlete stronger in a single maximal repetition. It means less of the working capacity is lost as time passes.
In competition, that difference can be enormous. The advantage may not be one extra kilogram on a deadlift. It may be the ability to access 95 percent of known capacity after a brutal event while another athlete has fallen to 80 percent.
Oxidative metabolism and technique under fatigue
As fatigue rises, technique deteriorates. Steps shorten, the trunk moves, grip opens and breathing rhythm breaks. Sometimes the problem looks technical, but the cause is metabolic. If the athlete cannot produce and restore enough ATP between contractions, motor control becomes harder to maintain.
A strong oxidative system can therefore appear indirectly in technique. Not because mitochondria directly control trunk position, but because they help provide the energy required to repeat well-executed movement.
When conditioning becomes a problem
Adding conditioning should improve total performance, not create an athlete who is exhausted in every direction. If strength falls persistently, sleep worsens, soreness lingers and key training days become weak, total conditioning dose may be too high.
At that point, more willpower is not the answer. Load management is. A strongman must weigh stimulus against cost and preserve enough recovery reserve for the adaptations that matter most.
A practical model for developing oxidative capacity
During a general training period, a reasonable structure might include one or two controlled oxidative sessions plus one specific conditioning session, depending on the athlete and calendar. This is a structural example, not a universal prescription.
One session can use easy-to-moderate continuous work. Another can use controlled intervals. The specific session can use sleds, farmer carries, sandbags or other implements, but at a volume low enough that every week does not become a competition.
How do you know the oxidative engine is improving?
There is no single perfect test for every component. In practical sport, you can look for faster recovery of heart rate and breathing, better ability to repeat efforts at the same output, less breathlessness for the same workload and longer preservation of technique.
Also watch what does not happen. Conditioning should not repeatedly destroy deadlift, squat, overhead or event-day performance. Metabolic progress is valuable when it translates into greater ability to perform the sport itself.
Mitochondria on competition day
Before the first event, the energy system is prepared. During the event, ATP is consumed. After the event, mitochondria work on recovery. Then comes the second event. Then the third. As the day progresses, the ability to recover between bursts becomes an increasingly visible part of performance.
In a five- or six-event competition, the winner is not always the athlete with the highest raw strength. Sometimes it is the athlete who can access enough of that strength every time the starter calls.
What a strongman should remember
Mitochondria are energy factories and metabolic hubs, not simple batteries. Carbohydrates and fats can feed oxidative metabolism. NADH and FADH2 carry electrons to the respiratory chain. The proton gradient powers ATP synthase. Oxygen is the final electron acceptor. Mitochondrial capacity adapts to training. And the strongman connection is direct: this infrastructure supports prolonged work, repeated explosive efforts and recovery between events.
Conclusion: the power plant nobody sees
The mitochondrion never appears in competition photographs. It does not lift the stone, push the sled or cross the finish line. Yet inside every active muscle fiber, it works continuously to support ATP production and to make recovery possible.
For strongman, the goal is not to turn the athlete into an endurance specialist. The goal is to build enough oxidative infrastructure for strength to be repeatable. The first explosion shows how strong you are. The second, third and fifth show how well you manage your energy.
The phosphagen system delivers the immediate strike. Glycolysis keeps intense work moving. The mitochondria support longer-term energy production and work quietly in the background of recovery. There is no single strongman engine. There is an entire factory.
Quick glossary
Mitochondrion: the organelle where much oxidative metabolism occurs. Acetyl-CoA: a central molecule that enters the Krebs cycle. NADH and FADH2: electron carriers that feed the respiratory chain. Respiratory chain: a system of protein complexes in the inner mitochondrial membrane. Proton gradient: an electrochemical difference used to power ATP synthesis. ATP synthase: the enzyme complex that uses the proton gradient to produce ATP. Mitochondrial biogenesis: processes through which cells build and remodel mitochondrial infrastructure. PGC-1α: an important regulator of oxidative adaptation.
Editorial note: this material is educational and does not replace medical assessment or individualized advice from a physician, physiologist or sports dietitian. Conditioning should be adapted to the athlete’s level, goals, injury history and total training load.
This is Episode 5 of “The Strongman Metabolism” series. The next natural step is a detailed examination of energy substrates, with carbohydrates, fats and proteins and how their availability changes performance in a strength athlete.
More From The Journal
Training
The Science of Strongman Training - Episode X: Competition Programming
How to build a complete Strongman competition preparation block: calendar, events, volume, intensity, specificity, simulations, autoregulation, tapering and fatigue management.
Training
The Science of Strongman Training - Episode IX: Peaking
Peaking in Strongman: how to turn months of training into maximal competition performance by reducing fatigue, preserving adaptations and managing specificity.